Master MCAT genetics and evolution concepts with high-yield explanations, practice questions, and detailed answers to boost your test performance.

(Note: This guide is part of our MCAT Biology series.)
Table of Contents
Part 1: Introduction to genetics and evolution
Part 2: Mendelian genetics
a) Chromosomes
b) Laws of Mendelian genetics
c) Dominance and recessivity
d) Punnett squares
Part 3: Non-Mendelian Genetics
a) Sex-linked genetics
b) Exceptions to complete dominance
c) Genetic linkage
d) Extranuclear inheritance
Part 4: Evolution
a) Natural selection
b) Genetic drift
c) Hardy-Weinberg equilibrium
Part 5: High-Yield Terms
Part 6: Passage-Based Questions and Answers
Part 7: Standalone Questions and Answers
-----
Part 1: Introduction to genetics and evolution
How do our cells know what to do and what to become? Genes play a large role in our development and function and dictate a large portion of what happens in our bodies. Thus, it is important to understand genetics and how differences in individuals with different genetic makeups can drive larger population changes.
Throughout the guide, several key terms will be emphasized in bold. At the end of the guide, there are also several MCAT-style questions that can be used to test your knowledge.
Receive Your Free MCAT Question of the Day
Get every last bit of practice in before test day with a free MCAT question delivered straight to your inbox daily.
-----
Part 2: Mendelian genetics
a) Chromosomes
In most cells, genetic information is stored as DNA packaged in the form of chromosomes. (To learn more about the genetic molecules, be sure to refer to our guide on DNA.)
Prokaryotes are organisms without any membrane-bound organelles. Prokaryotic cells include archaea and bacteria. Within these organisms, the DNA molecule is usually circular and unprotected within the cytoplasm.
Eukaryotes are organisms with membrane-bound organelles. These include animals, plants, fungi, and protists—thus including humans as well. Eukaryotic cells contain linear chromosomes of DNA scaffolded in proteins. This DNA is stored in a cell’s nucleus, and each chromosome consists of one single DNA molecule.

Figure 1 Prokaryotic and eukaryotic chromosomes.
DNA that is transcriptionally active, or relaxed, is referred to as euchromatin. DNA that is transcriptionally inactive, or condensed, is referred to as heterochromatin. In a mature eukaryotic cell, chromosomes are formed by pairs of chromatids that are joined at a centromere. Each chromatid has a long and a short arm. Telomeres are located at the end of each chromatid and are regions of high G-C content. These regions are used as buffer regions to prevent the shortening of the DNA molecule during replication and thus shorten with each round of cell replication. When a number of cell divisions known as the Hayflick limit are reached, the cell can no longer safely replicate and will undergo cell death.

Figure 2 Structure of chromosomes.
Karyotypes visualize the chromosomes in an organism’s cell. Karyotypes are usually performed in a laboratory, where chromosomes are usually stained under the microscope: sometimes with fluorescent dyes to differentiate the different regions of the chromosome. Photographs of an individual’s condensed chromosomes are taken and digitally manipulated to arrange individual chromosomes by decreasing size.

Figure 3 Steps of karyotyping.
Karyotyping is useful in detecting chromosomal anomalies that can cause diseases. Chromosomal abnormalities include aneuploidy (the absence of a chromosome or the presence of an extra one), or structural abnormalities (changes in one or more individual chromosomes). Examples of aneuploidy include trisomy 21, also known as Down syndrome, in which an extra copy of chromosome #21 is inherited by an offspring. Structural abnormalities can occur in a wide range of varieties, including the following:
Deletion: in which a segment of a chromosome is missing
Duplication: in which a segment of a chromosome is repeated on the same arm
Inversion: in which two regions on the same chromosome are swapped
Substitution: in which a region on one chromosome is inserted into the arm of another chromosome
Translocation: in which the terminal regions of two different chromosomes are swapped
Additional changes in DNA, also known as a mutation, can occur on a smaller scale. Mutations generally arise as a result of the presence of mutagens in the environment.
A point mutation is a result of the change of a single nucleotide within the DNA sequence. The nucleotide (A, C, T, or G) may be swapped out for another nucleotide at the same location.
A frameshift mutation is a result of either a deleted or inserted set of nucleotides that alter the reading frame of the sequence. (Recall that three-letter codons are translated by the ribosome into amino acids; changing the location of the frame can alter the translated amino acids.)
A mispairing mutation results from the separation and failed re-attachment of two strands of DNA. This mutation results in the mispairing of individual DNA nucleotides: for instance, A failing to bind with T or C failing to bind with G.
The same locus or gene can also give rise to multiple different phenotypes. For instance, a single gene encoding eye color can encode one of multiple different eye colors: blue, brown, green, and so forth. Such a mutation is referred to as a polymorphism.
Humans normally have 23 pairs of chromosomes in each cell: each parent contributes one set of 23 chromosomes. Thus, a normal human karyotype should contain 46 chromosomes. The human genome is composed of 23 pairs of homologous chromosomes, implying that each paternal and maternal chromosome contains the same sets of genes. Humans and most other mammals are diploid organisms, in which ploidy refers to the number of sets of chromosomes found in a cell.
A minor exception to this rule is the 23rd pair of chromosomes, known as the sex chromosomes. These chromosomes determine the genetic sex of an individual: females have 2 X chromosomes (karyotype XX), while a male has an X chromosome and a smaller Y chromosome (karyotype XY). The other 44 chromosomes are known as autosomes and are numbered from pairs 1 to 22.

Figure 4 An example of a human karyotype.
If all humans have the same set of chromosomes that carry the same sets of genes, how do our individual differences arise? One of the most important sources of variation lies in the concept of alleles, or gene variants. While members of the same species have the same genes, these genes can vary in DNA sequence between individual members and even between the two copies within a diploid cell. Multiple alleles can exist for a single gene, each with potentially different characteristics. Each human cell carries at least 2 alleles of each gene, and these can either be identical or unique.
While all alleles for a gene are found at the same position, or locus (plural: loci) on a chromosome, variations in gene sequences confer different characteristics for gene activity. It is this complex interplay between the different genetic profiles of alleles, or genotypes, that leads to the different physical characteristics, or phenotypes, of different individuals.
b) Laws of Mendelian genetics
Gregor Mendel, a 19th century monk, conducted many important studies on the genetic inheritance of traits using pea plants. Mendel proposed a number of laws on the heredity of traits, which have since been refined and confirmed by modern discovery. Several of Mendel’s laws dictate the events that occur during meiosis, a key step during sexual reproduction in which haploid gametes are formed.
The law of segregation states that the two allelic copies of genes in a diploid organism are equally segregated into gametes, such that the two gametes that are formed both receive one of the pairs of alleles. Since diploid organisms carry two copies of all genes, this applies to all genes present during meiosis I: alleles are equally distributed to daughter gametes from a dividing mother cell.
The law of independent assortment states that the separation of the alleles of one gene occurs separately and uniquely from the separation of alleles of another gene. Thus, different genes pass on alleles to gametes without affecting the assortment of other genes. The independent assortment of homologous chromosomes prior to anaphase allows alleles to be differently distributed into their respective daughter cells, creating variation within the gametes themselves.

Figure 5 The Law of Segregation and Law of Independent Assortment.
c) Dominance and recessivity
Recall that an individual’s genotype refers to the genetic alleles that make up a trait, while its phenotype is the physical expression of the trait. When a diploid organism carries two identical alleles of a gene, it is considered to be homozygous. The presence of two different alleles indicates heterozygosity for that gene. When two different alleles exist in an individual, their relationship will determine the phenotypic expression of such genes.
Alleles can be dominant or recessive. Dominant alleles exert a stronger phenotypic effect and will mask the effects of the recessive allele if both are present in a heterozygote. This means that to express a recessive phenotype, the organism must possess two copies of the recessive allele (e.g., a homozygous recessive genotype). In contrast, the dominant phenotype could be expressed with just one copy of the allele or two (e.g., a heterozygous or homozygous dominant genotype). When a phenotypic trait is expressed with only one inherited copy of a dominant allele, that trait is said to possess complete dominance.
Table 1 Genotype and Phenotype for Given Alleles
| Inherited alleles | Genotype | Phenotype | ||
|---|---|---|---|---|
Recall that genes encode proteins, and proteins determine function. Thus, a recessive gene may often result in a loss of function for the respective protein. Often, having both recessive alleles can be potentially pathological, which is why some diseases result from a homozygous recessive genotype. An example of one such disease is cystic fibrosis, which arises due to mutations in the CFTR gene. Those that carry both mutated (recessive) alleles suffer from cystic fibrosis, while those that carry one normal allele, or a wild-type allele, and a recessive allele do not suffer the same condition because of the dominant wild-type allele’s masking effects. Instead, this heterozygous individual is known as a carrier of the disease: one who can pass on the recessive allele to their offspring but does not express the recessive phenotype themselves.
d) Punnett squares

Figure 6 An example of a monohybrid cross.
A dihybrid cross is a little more complex as it involves the allele types for two different genes instead of one. Since each parent can contribute 1 of 2 alleles per gene in the gamete, each parent can contribute 2 x 2 = 4 potential gametes with respect to 2 genes, and thus a 4x4 Punnett square with 16 potential outcomes is used.
Consider a dihybrid cross in which Parent 1 carries the AaBb genotype, while Parent 2 also carries the AaBb genotype.
Parent 1 carries two different alleles (A and a) at the first gene locus. Thus, a gamete formed by Parent 1 will have one of these two alleles (A or a). Additionally, Parent 1 carries two different alleles (B and b) at the second gene locus. Thus, a gamete formed by Parent 1 will also carry one of these two alleles (B or b).
The same exercise can be performed for Parent 2. Parent 2 carries two different alleles (A and a) at the first gene locus. Thus, a gamete formed by Parent 1 will have one of these two alleles (A or a). Additionally, Parent 2 carries two different alleles (B and b) at the second gene locus. Thus, a gamete formed by Parent 2 will also carry one of these two alleles (B or b).

Figure 7 An example of determining the four possible gametes contributed by a single parent.
After determining the possible gametes contributed by each parent, the Punnett square is created. The possible gametes are written across the top row and leftmost column, and genotypes of individual offspring can be written by combining the genotypes of gametes from each parent.

Figure 8 An example of a dihybrid cross.
The frequencies of individual genotypes resulting from the Punnett square can be used to predict the frequencies of genotypes in the offspring. In this example:
The genotype AABB appears once. Thus, the probability of randomly receiving an offspring that is homozygous dominant in both gene A and gene B is 1/16.
The genotype AABb appears twice. Thus, the probability of randomly receiving an offspring that is both homozygous dominant in gene A and heterozygous in gene B is 2/16, or ⅛.
The genotype AaBB appears twice. Thus, the probability of randomly receiving an offspring that is both heterozygous in gene A and homozygous dominant in gene A is 2/16, or ⅛.
The genotype AAbb appears once. Thus, the probability of randomly receiving an offspring that is both homozygous dominant in gene A and homozygous recessive in gene A is 1/16.
The genotype AaBb appears four times. Thus, the probability of randomly receiving an offspring that is heterozygous in both genes is 4/16, or ¼.
The genotype Aabb appears two times. Thus, the probability of randomly receiving an offspring that is both heterozygous in gene A and homozygous recessive in gene B is 2/16, or ⅛.
The genotype aaBB appears once. Thus, the probability of randomly receiving an offspring that is both homozygous recessive in gene A and homozygous dominant in gene B is 1/16.
The genotype aaBb appears twice. Thus, the probability of randomly receiving an offspring that is both homozygous recessive in gene A and heterozygous in gene B is 2/16, or ⅛.
The genotype aabb appears once. Thus, the probability of randomly receiving an offspring that is homozygous recessive in both gene A and gene B is 1/16.
Note that to predict the frequency of expressed traits in the offspring, these genotypes must be decoded to their respective phenotypes. In this example,
The probability of receiving an offspring that is dominant in traits encoded by both gene A and gene B is 9/16.
The probability of receiving an offspring that is both dominant in a trait encoded by gene A and recessive in a trait encoded by gene B is 3/16.
The probability of receiving an offspring that is both recessive in a trait encoded by gene A and dominant in a trait encoded by gene B is 3/16.
The probability of receiving an offspring that is recessive in traits encoded by both gene A and gene B is 1/16.
Punnett squares are used to estimate the potential makeup of the offspring pool when two organisms with known genotypes are crossed. Punnett squares can also be used in reverse to determine the genotype of an organism in what is called a test cross. A test cross, sometimes referred to as a back cross, is usually used to determine whether an organism is a dominant homozygote or a heterozygote and involves crossing the organism of interest with a homozygous recessive individual. The proportion of offspring displaying dominant or recessive phenotypes can then be used to determine the genotype of the organism of interest.
Consider the following example of a test cross with flowers. The dominant phenotype is a blue color, while the recessive phenotype is a white color. To determine the unknown genotype of a blue flower, it is bred with a homozygous recessive (white-colored) individual.
After the two parents are bred, the phenotypes of the offspring are counted and compared against predictions that are made from Punnett squares.

Figure 9 An example of a test cross.
Test crosses may be performed between individuals of successive generations. In this case, the parental (P) generation is said to yield the F1 (“first filial”) generation. Crosses between individuals from the F1 generation yield the F2 (“second filial”) generation.
-----
Part 3: Non-Mendelian genetics
a) Sex-linked genetics
Not all allelic relationships follow the Mendelian laws that we previously discussed. For example, unique inheritance patterns occur when the gene of interest is found on the sex chromosome (chromosome number 23). These genes are known as sex-linked genes.
Because the human X chromosome is much larger than the Y chromosome and therefore contains more genes, the MCAT will usually focus on genes that are found on the X chromosome. Such genes follow an X-linked inheritance pattern. While the basic principles of dominance and recessivity still apply, X-linked conditions affect males and females differently due to the difference in the numbers of alleles that are present in the two sexes.
X-linked recessive traits are commonly tested on the MCAT. Recall that females possess two X chromosomes, while males only possess one X chromosome. Thus, while a female requires both copies of alleles to be recessive to display the recessive trait, the male only requires the sole X-chromosome to have the recessive allele to display the trait. In addition, female carriers can pass on recessive X-linked alleles to both sons and daughters, while diseased males can only pass on the recessive X-linked allele to a daughter. (This is because any sons must necessarily receive the father’s Y chromosome). This makes males more likely to suffer from X-linked recessive conditions than females, such as red-green color blindness.
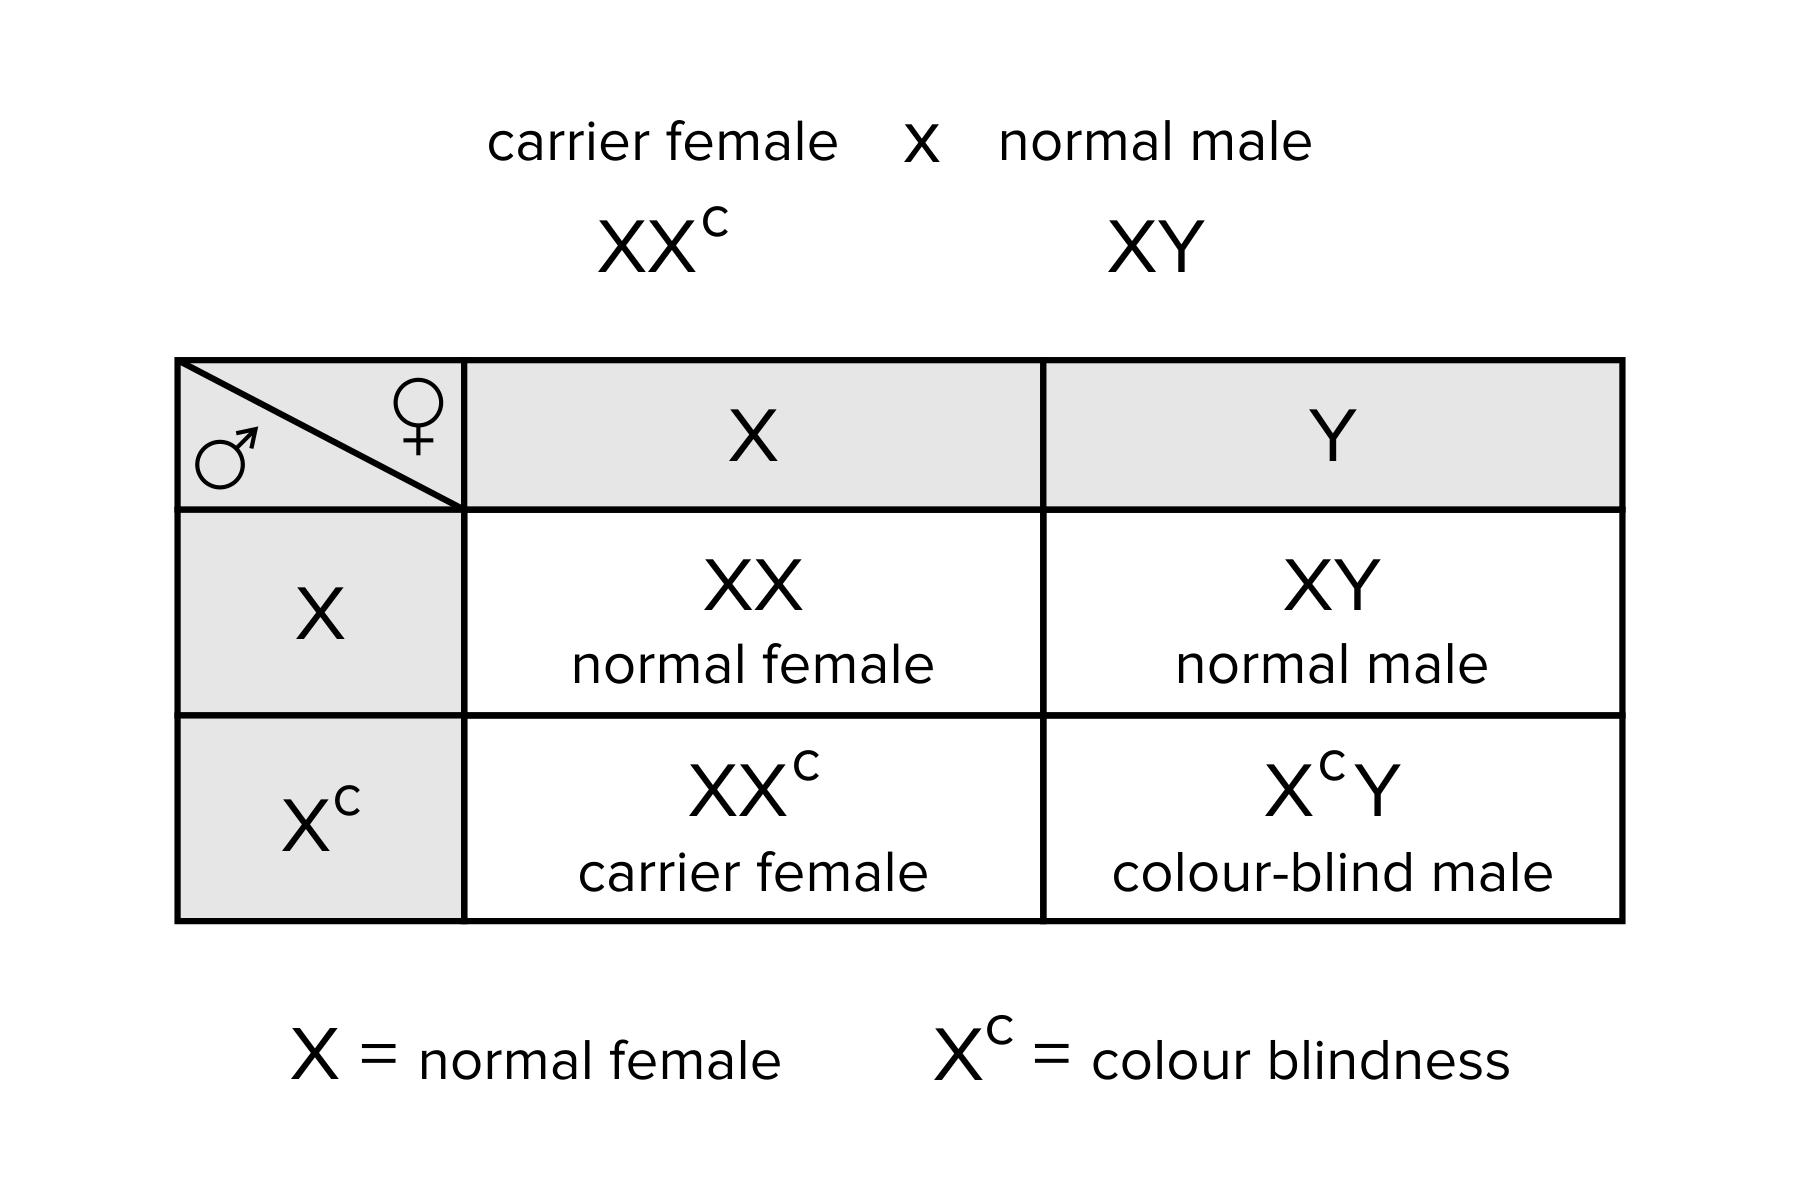
Figure 10 A test cross for an X-linked recessive condition.
X-linked dominant traits and Y-linked traits also exist. When examining sex-linked traits, one must consider not only the basic rules of allelic relationships but also bear in mind the differences in copy numbers in males and females.
b) Exceptions to complete dominance
Many genes follow the dominant/recessive relationship described earlier. However, other genes do not. Codominance occurs when two different alleles’ respective phenotypes are expressed at the same time. Neither allele’s phenotypic characteristic masks or affects the expression of the other allele’s phenotypic characteristic. This occurs in traits such as blood type, where the inheritance of both a blood type “A” allele and a blood type “B” allele results in the expression of both phenotypes: an AB blood type.
Incomplete dominance occurs when the presence of a dominant and a recessive allele creates a phenotype that is different from either dominant or recessive phenotypes. The resulting phenotype is usually an intermediate blend of the phenotypes found in the two different homozygotes. This can be seen in traits such as snapdragon color. While the dominant trait may be a red color and the recessive trait may be a white color, a heterozygous genotype results in an intermediate phenotype: a pink color.
The extent to which genotypes affect the phenotype is described by penetrance and expressivity. Penetrance describes the frequency of individuals within a population that actually display the predicted phenotype. Expressivity refers to the extent to which the related phenotypic trait is expressed in a single individual. To rephrase, penetrance is concerned with whether an individual who has a genotype also displays the resulting phenotype, while expressivity is concerned with how strongly the phenotype is expressed.
In the following illustrated example, assume that every individual (represented by a circle) possesses the same heterozygous genotype. The gene in question encodes for color, in which black is dominant and white is recessive. Despite the identical genotypes of each individual, the expressed phenotypes see high amounts of variance.

Figure 11 Penetrance and expressivity as demonstrated in a population where individuals are drawn as circles.
Classical Mendelian genetics assumes complete penetrance, implying that all members of a population that possess the genes for a trait will express the trait. In reality, reduced penetrance often occurs. In addition, variable expressivity describes how different members of a population with the same traits express them at a range of severities. In this context, expressivity is often described as narrow (limited) or broad (variable).
c) Genetic linkage
In our previous discussion on the law of independent assortment, it was stated that sets of genes located on different places on a chromosome would assort independently during meiosis.
This holds largely true for alleles of different genes on the same chromosome. Genes located far apart from one another are rarely inherited together because of genetic recombination during meiosis, in which homologous chromosomes in a cell exchange portions of DNA and thereby swap alleles. This is especially true for genes that are far apart, because recombination is more likely to occur at a site in between.
This does not fully apply to genes that are found close together on the same chromosome, or linked genes. Traits that are clustered in neighboring loci are more likely to be inherited together and therefore pose an exception to the law of independent assortment. Map units or centimorgans are a unit used to quantify the distance between two genes on the same chromosome. These quantities are related to the crossover frequency, which describes the frequency at which two genes are separately inherited.
This information can be provided through a technique known as gene mapping.
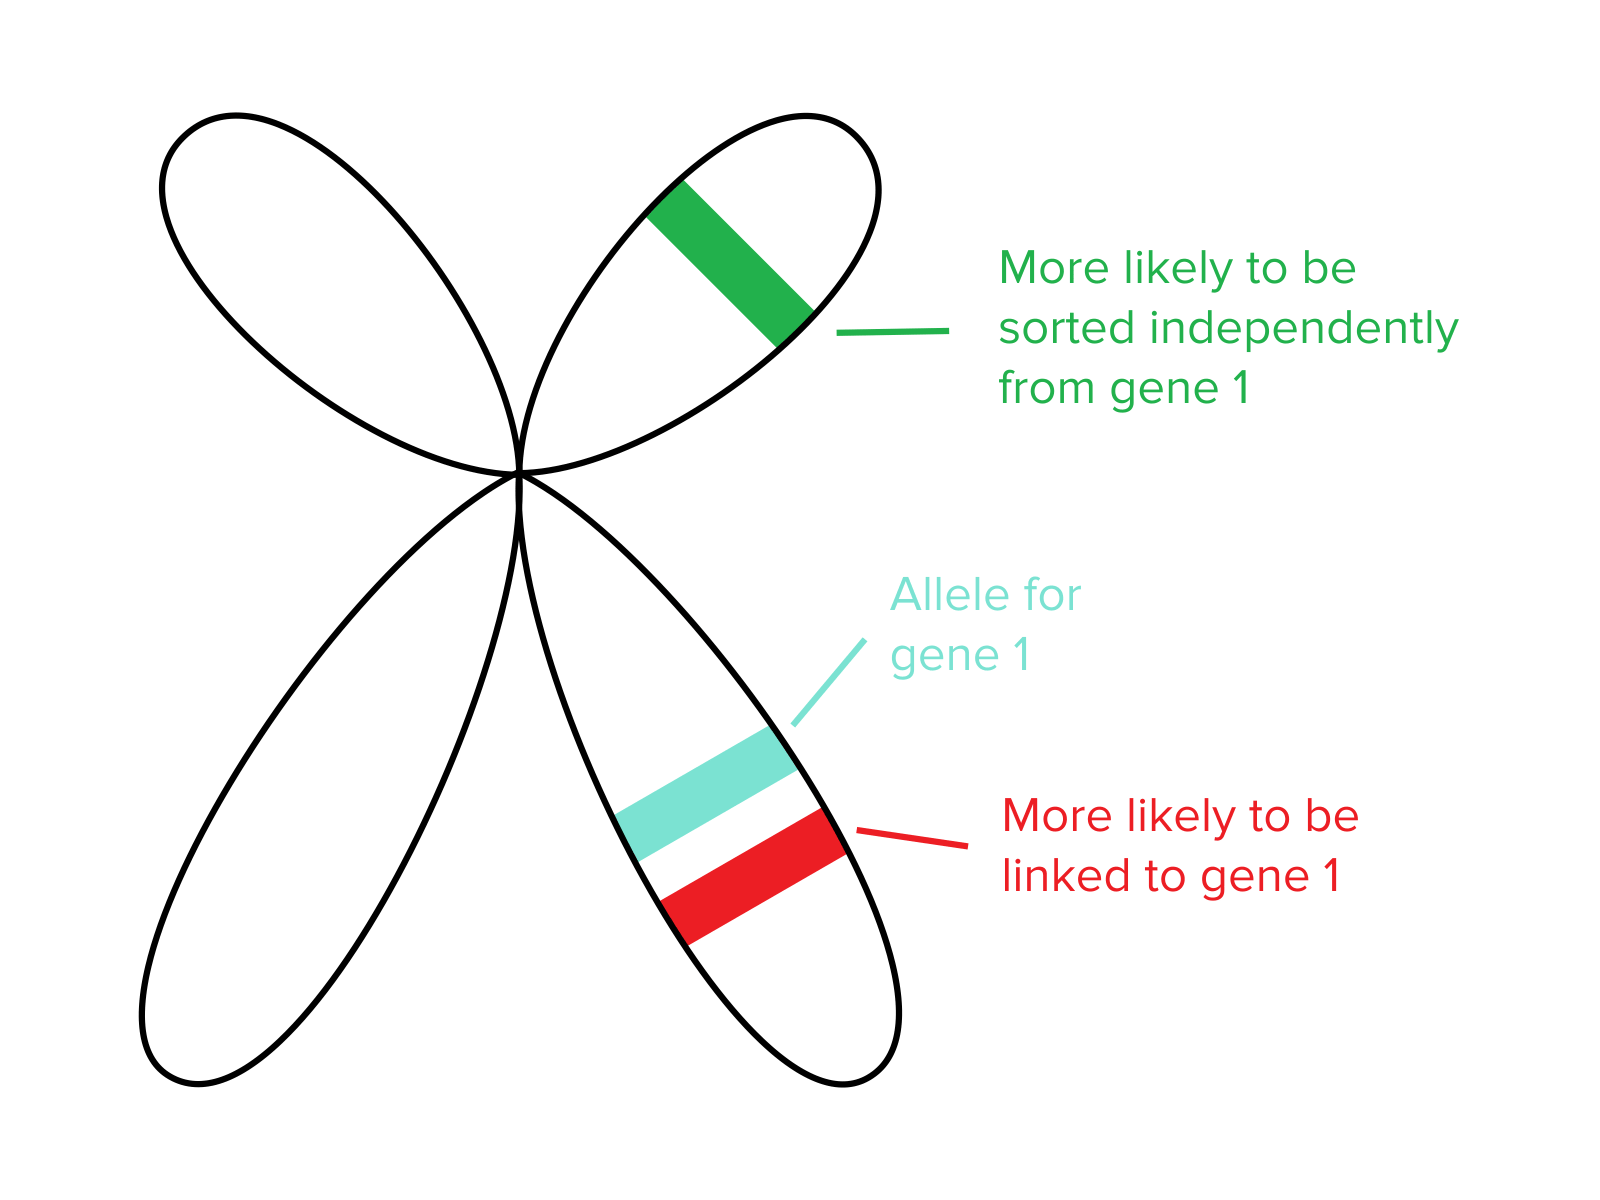
Figure 12 Genes that are located closer together are more likely to be linked together.
d) Extranuclear inheritance
Throughout this guide, we’ve discussed the inheritance of chromosomes and genetic information that exists within the nucleus of a cell. However, in certain eukaryotes, there is also genetic information that exists outside of the nucleus.
Certain organelles such as mitochondria and chloroplasts also contain fragments of genetic information. As these organelles are replicated and passed from parent to offspring, any DNA within these organelles can also be inherited.
In humans, this extranuclear inheritance can occur through maternal mitochondria. Recall that in early reproduction, a sperm fertilizes an ovum (or egg). This ovum is relatively large and contains all of the cytosol and organelles that will contribute to the developing organism. Since the maternal ovum contributes the vast majority of mitochondria within the new offspring, the new offspring will inherit any and all genetic material present within the mother’s mitochondria.
-----
Part 4: Evolution
a) Natural selection
Evolution is a major driver of change in a population and is most often driven by natural selection. Natural selection, often phrased as “survival of the fittest,” is the process through which individuals with traits that favor their survival and reproduction outcompete individuals less fitted to the living environment, eventually creating large-scale changes in the gene pool of the population.
In an environment that exerts selective pressure on a population—for instance, through food scarcity or predation—individuals with more adapted characteristics can more successfully produce offspring, the more adapted of which can then out-reproduce their counterparts in the next generation. This process of differential reproduction results in the increasing allele frequency of favorable alleles and their resultant adaptive traits in the population. When the selective pressure is changed, the same process will occur, this time favoring whatever genotypes produce individuals more suited to handle this new form of selection.
As a general rule of thumb, a population with higher allele diversity exhibits more successful differential reproduction. However, this diversity can change due to the presence of inbreeding or outbreeding. Inbreeding occurs as members within a population continue to mate and reproduce with one another; this decreases the variability of traits within a population, and thus decreases the success of the population. In contrast, outbreeding occurs as members of different populations encounter and mate with one another. This introduces new variability into the group, leading to an increase in reproductive fitness.
Note that trait selection can occur at several different levels. It can occur on an individual level, in which individuals with favorable traits are able to reproduce and pass on their traits to offspring. However, group selection can also occur, in which entire groups that perform favorable behaviors promote the reproductive success of the group as a whole. (Altruistic behaviors are a good example of group selection at play; while the reproductive success of individuals exhibiting the behavior may be diminished, these behaviors increase the fitness of the species as a whole.)
It is important to note that evolution is not the equivalent of natural selection. Natural selection is a mechanism by which a population evolves. However, evolutionary change in populations can also occur in other ways.
b) Genetic drift
Genetic drift is a mechanism of allele frequency change that is most prominent when a population faces no selective pressures. In the absence of selection, random mutations that give rise to new alleles can affect the population’s allele frequencies from one generation to the next.
These random mutations may arise in unfavorable mutations, which lower the genetic fitness of an individual and may decrease their chance of survival. Examples of deleterious mutations include inborn errors of metabolism: genetic disorders present at birth within an individual, which disrupt the production of key enzymes that are used in metabolic pathways. Individuals with such inborn errors may need to follow a specialized diet during their lifetimes. Such is the case with patients diagnosed with phenylketonuria, which results in a decreased ability to process phenylalanine.
Mutations may also result in favorable adaptations, which ultimately increase the genetic fitness of an individual. Mutations may also arise in the specialization of certain phenotypes: for instance, in the specialization of a bird’s beak to retrieve seeds from a pinecone. This specialization allows a species to occupy a particular ecological niche and benefit from certain resources that are otherwise unexploited.
New mutations may also arise from genetic leakage. Genetic leakage occurs as genes are transferred between species: through inter-species breeding (which may create an infertile hybrid offspring) or incorporating intracellular genetic products, such as mitochondrial DNA, into the species genome.
Although novel alleles may undergo elimination from the population due to such chance events, they may also persist and undergo fixation within the population. A trait is said to be particularly successful if its incidence within a population increases: that is, if more and more of the individuals in the population inherit the trait over time. When fixation occurs, the trait becomes a novel phenotype that is possible within the population. This process occurs in natural selection, but in this latter case, the fate of the novel alleles is determined by whether they confer positive or negative selective advantages to the new mutants.
The effects of genetic drift are most pronounced when coupled with major changes in the population makeup. Catastrophes that greatly reduce a population’s size will randomly remove variant alleles via the bottleneck effect, in which the relatively small pool of survivors is left to pass on a lower diversity of genes onto offspring. Small populations that branch off the main population to form a new colony suffer from the founder effect. Both changes result in decreased allelic diversity, and the smaller population size renders the new population more susceptible to the further loss of alleles due to genetic drift. For these reasons, a high amount of genetic diversity within a population is usually favored.

Figure 13 The bottleneck and founder's effects.
These evolutionary pressures can gradually result in speciation, or the arising of a new species. Speciation is said to occur when two genetically distinct lineages are formed. Members of these different lineages would not be able to mate and produce fertile offspring.
The molecular clock is a theoretical method of dating the evolutionary age of a species based on the frequency of allele changes that have occurred. In other words, the amount of evolutionary time that has passed can be roughly determined by the number of random, gradual changes that have occurred in the genome of a particular species. The number of differences in genetic traits between two species is said to be correlated with the time since their evolutionary divergence; thus, the higher the degree of genetic difference between two species, the longer ago they are assumed to have diverged.
c) Hardy-Weinberg equilibrium
How do we determine the changes of allele frequency in a population over time? To determine if significant large-scale changes in allele frequency are made, statistical methods must be employed. Biometry refers to the statistical analysis of biological data and can be useful in determining when natural selection is occurring.
When the allele frequencies within a population remain stable over time, the population is not evolving and is said to be in Hardy-Weinberg equilibrium. Several conditions must be satisfied for Hardy-Weinberg equilibrium to be met:
1. Random mating of individuals (no sexual selection)
2. All phenotypes have equal viability and reproductive success (no natural selection)
3. Populations are (infinitely) large
4. No gene flow (no migration)
5. No new mutations arise (no genetic drift)
In most real-world situations, these conditions are strictly hypothetically and highly unlikely to occur. If any of the five conditions are not met, then allele frequencies will change, and population evolution may occur.
The Hardy-Weinberg equations are two sets of equations that describe the allele frequencies for a trait that can be either dominant or recessive. Here, p is a variable that represents the frequency of the dominant allele in a population, while q is a variable that represents the frequency of the recessive allele in a population.
In any population with two alleles for a gene, the allele frequencies obey the equation:
p + q = 1
- p2 represents the frequency of homozygous dominant genotypes
- 2pq represents the frequency of heterozygous individuals
- q2 represents the frequency of homozygous recessive genotypes.
These two equations allow for the estimation of any allelic frequency if any one genotype frequency is known, or vice versa. For a population in Hardy-Weinberg equilibrium, the allele and genotype frequencies will remain constant over generations.
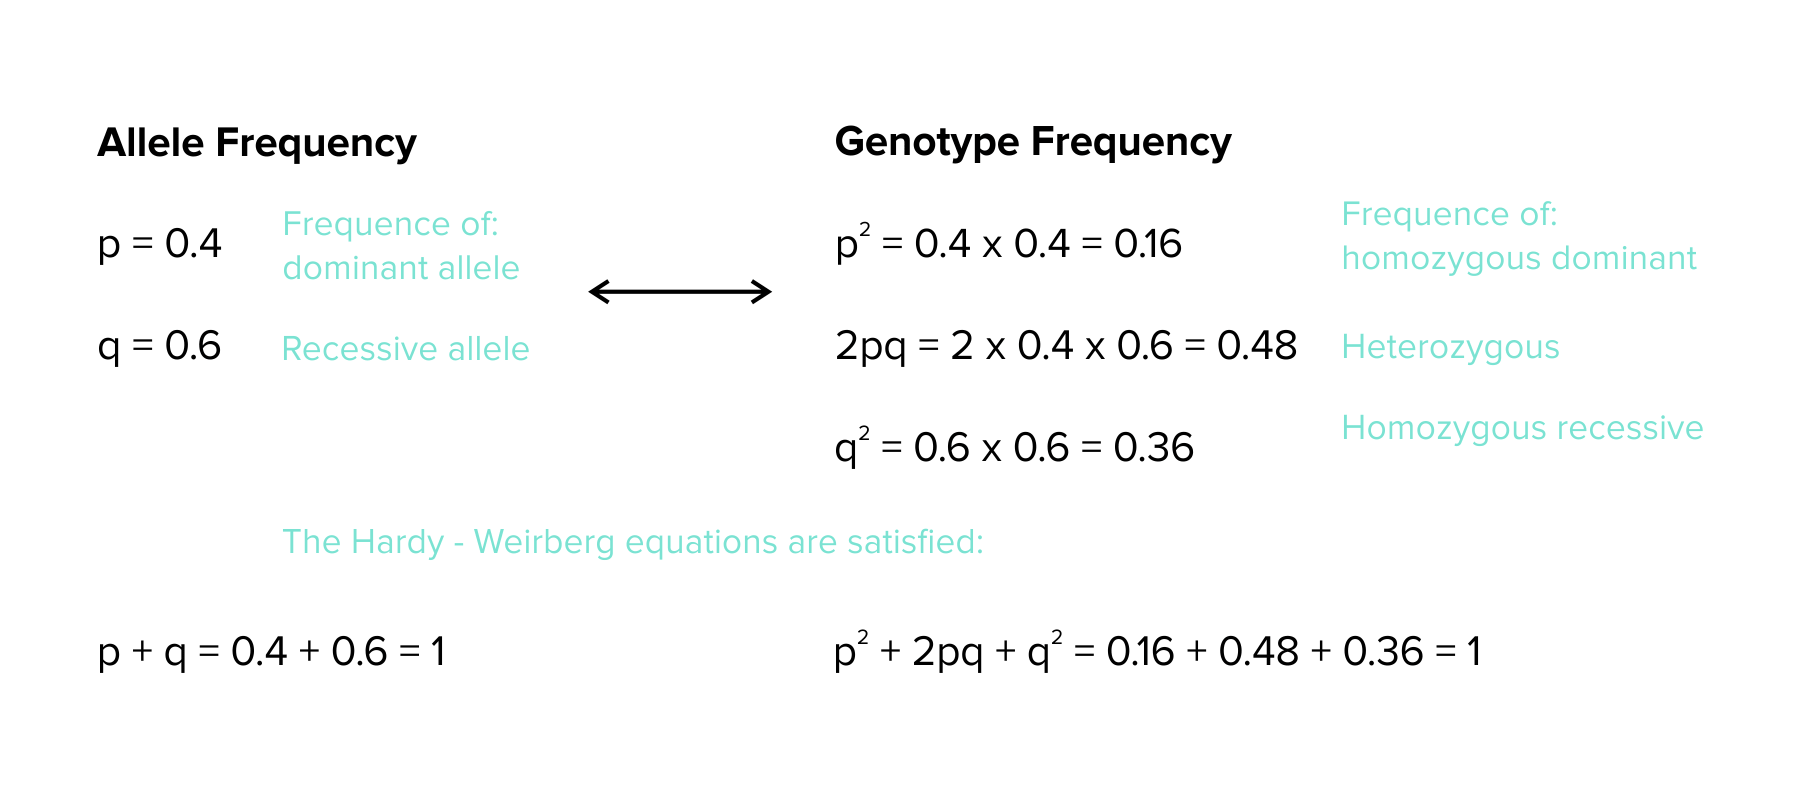
Figure 14 An example of using the Hardy-Weinberg equations.
-----
Part 5: High-yield terms
Chromosome: stored and packaged DNA
Prokaryotes: organisms without any membrane-bound organelles
Eukaryotes: organisms with membrane-bound organelles
Telomeres: regions of high G-C content at the end of each chromatid
Karyotypes: images that visualize the chromosomes in an organism’s cell
Aneuploidy: the absence of a chromosome or the presence of an extra one
Structural abnormalities: changes in one or more individual chromosomes
Ploidy: the number of sets of chromosomes found in a cell.
Sex chromosomes: the 23rd pair of chromosomes, which determines genetic sex
Autosomes: the 1st through 22nd pairs of chromosomes, which do not determine genetic sex
Locus: the position, or location, of a gene on a chromosome
Genotype: an inherited genetic profile for a trait; determines a phenotype
Phenotype: an expressed physical characteristic; determined by a genotype
Law of segregation: states that the two allelic copies of genes in a diploid organism are equally segregated into gametes, such that the two gametes that are formed both receive one of the pairs of alleles
Law of independent assortment: states that the separation of the alleles of one gene occurs separately and uniquely from the separation of alleles of another gene
Homozygosity: presence of two identical alleles at the same gene
Heterozygosity: presence of two different alleles at the same gene
Carrier: one who can pass on the recessive allele to their offspring but does not express the recessive phenotype themselves.
Monohybrid cross: analysis of potential combinations of parental alleles with respect to one gene
Dihybrid cross: analysis of the allele types for two different genes, instead of one
Test cross: crossing the organism of interest with a homozygous recessive individual to determine whether an organism is a dominant homozygote or a heterozygote
X-linked recessive disorders: expressed in females that inherit two recessive X-linked alleles and males that inherit one X-linked recessive allele
Codominance: occurs when two different alleles’ respective phenotypes are expressed at the same time
Incomplete dominance: occurs when the presence of a dominant and a recessive allele creates a phenotype that is different from either dominant or recessive phenotypes
Penetrance: the proportion of individuals within a population that actually display the predicted phenotype
Expressivity: extent to which the related phenotypic trait is expressed in a single individual
Linked genes: genes that are found close together on the same chromosome and are thus more likely to be inherited together
Map units: unit used to quantify the distance between two genes on the same chromosome
Natural selection: process through which individuals with traits that favor their survival and reproduction outcompete individuals less fitted to the living environment
Genetic drift: random, spontaneous allele frequency change that is most prominent when a population faces no selective pressures
Bottleneck effect: low genetic variation that results when a relatively small pool of survivors are left to pass on a lower diversity of genes onto offspring after a catastrophe
Founder effect: low genetic variation that results when small populations that branch off the main population to form a new colony
Molecular clock theory: theoretical method of dating the evolutionary age of a species that states the higher the degree of genetic difference between two species, the longer ago they are assumed to have diverged
Hardy-Weinberg equilibrium: theoretical state in which no allele frequencies change
-----
Part 6: Passage-based questions and answers
Human societies living in highlands and mountainous areas encounter many inhospitable factors within their environment. Ancient and modern societies living in Central Andes (above 2500 meters above sea level) are directly affected by low oxygen pressure, which may lead to hypobaric hypoxia and cold temperatures.
Descendants of ancient Andean populations display traits that include elevated concentrations of hemoglobin, thoracic expansion, increased lung capacities, and higher levels of pulmonary arterial pressure. These traits are theorized to ameliorate the negative effects of hypoxia that may be encountered at high elevations.
These traits are considered to have arisen through one of two possible paths: one in which exposure to low oxygen levels promoted adaptation through natural selection, and one in which a previously existing phenotype enabled humans to live and thrive in an otherwise hypoxic environment. Three-different single-nucleotide polymorphisms (SNPs) in two different candidate genes (NOS3: rs1799983 G>T; EGLN1: rs1769792 T>G, rs1769813 A>T) were identified as targets for analysis.
Researchers analyzed paleogenomic data from 150 prehistoric individuals who had lived between 8500 to 600 years before the present year. These individuals were further identified to have lived along the ancient coast (a low-altitude environment) or in the ancient highlands (a high-altitude environment). Multiplex-PCR and single base extension assays were used to genotype these three altitude adaptation-associated SNPs.
Table 1 Allele and genotype frequencies determined for the NOS3, EGLN1 and BAZ4 SNPs.
| Age in Generations (Tmod - n) | n | NOS3(rs1799983) | EGLN1(rs1769792) | EGLN1(rs1769813) | ||||
|---|---|---|---|---|---|---|---|---|
| Ancient Coast | ||||||||
| Ancient Highlands | ||||||||
Based on the results of computer simulations and statistical analysis, the researchers concluded that natural selection was ongoing during the investigated timespan and was thus responsible for the genetic diversity of Andean highlanders.
CREATOR AND ATTRIBUTION PARTY: FEHREN-SCHMITZ, L., GEORGES, L. ANCIENT DNA REVEALS SELECTION ACTING ON GENES ASSOCIATED WITH HYPOXIA RESPONSE IN PRE-COLUMBIAN PERUVIAN HIGHLANDERS IN THE LAST 8500 YEARS. SCI REP 6, 23485 (2016). HTTPS://DOI.ORG/10.1038/SREP23485. THE ARTICLE’S FULL TEXT IS AVAILABLE HERE: HTTPS://WWW.NATURE.COM/ARTICLES/SREP23485. THE ARTICLE IS NOT COPYRIGHTED BY SHEMMASSIAN ACADEMIC CONSULTING. DISCLAIMER: SHEMMASSIAN ACADEMIC CONSULTING DOES NOT OWN THE PASSAGE PRESENTED HERE. CREATIVE COMMON LICENSE: HTTP://CREATIVECOMMONS.ORG/LICENSES/BY/4.0/. CHANGES WERE MADE TO ORIGINAL ARTICLE TO CREATE AN MCAT-STYLE PASSAGE.
Question 1: The SNP mutations investigated in this study were most likely the result of:
A) Bottleneck effect
B) Founder’s effect
C) Genetic drift
D) Migration
Question 2: What is the expected number of individuals heterozygous for the rs1769813 mutation in a population of 1000 individuals living among the ancient coast?
A) 240
B) 480
C) 450
D) 360
Question 3: Assume that some individuals who inherit these SNPs express increased cardiac vascularization and increased arterial oxygen saturation. Which of the following can be concluded?
A) Individuals in this population have inherited structural abnormalities
B) The population is no longer in Hardy-Weinberg equilibrium
C) The trait must be sex-linked recessive
D) The trait must be codominant
Question 4: Upon additional analysis, researchers discover that the two EGLN1 mutations are often inherited from each other. Which of the following laws has been shown to be violated?
A) Law of independent assortment
B) Law of expressivity
C) Law of segregation
D) Law of parsimony
Question 5: Suppose that compared to the modern population, all ancient peoples who lived in the highlands displayed higher tolerance to hypobaric hypoxia. However, individuals within the ancient population displayed high amounts of variance to this tolerance. This trait is best described as expressing:
A) Complete penetrance and broad expressivity
B) Complete penetrance and narrow expressivity
C) Incomplete penetrance and broad expressivity
D) Incomplete penetrance and narrow expressivity
Answer key for passage-based questions
Answer choice C is correct. Single-nucleotide polymorphisms (SNPs) are mutations at a single DNA nucleotide within the genetic code. These mutations occur randomly and at chance (choice C is correct). The bottleneck effect and founder’s effect explain the drastic changes in frequency that may be present after a migration event or natural disaster but does not apply to the onset of genetic mutations (choices A and B are incorrect). Migration is an event that refers to the movement of individuals across a geographic region (choice D is incorrect).
Answer choice B is correct. From the information presented in the table, the frequency of the A allele is approximately p = 0.6, while the frequency of the T allele is approximately q = 0.4. These frequencies appear to be stable over time. Based on the Hardy-Weinberg equations, the frequency of heterozygous individuals can be calculated as 2pq = 2 * 0.6 * 0.4 = 0.48. Thus, in a population of 1000 people, there should be 480 heterozygous individuals.
Answer choice B is correct. To meet the Hardy-Weinberg conditions, a population cannot experience changes in allele frequency. Thus, the population cannot undergo natural selection (choice B is correct). A structural abnormality is a change in a localized region of one or more chromosomes; there is not enough evidence that this has occurred (choice A is incorrect). While there is some evidence that this trait is recessive, there is not enough evidence that this trait follows non-Mendelian genetics (choices C and D are incorrect).
Answer choice A is correct. The genes are found to be linked. Genetic linkage is most often due to the close physical proximity of genes on a chromosome, meaning they are less likely to assort independently of each other (choice A is correct). Expressivity refers to the extent to which an inherited phenotypic trait is displayed in a single individual (choice B is incorrect). Segregation states that alleles are divided into gametes such that each gamete receives an equal number of alleles (choice C is incorrect). The law of parsimony is used to build evolutionary trees and states that the tree with the fewest amount of evolved traits is most likely correct (choice D is incorrect).
Answer choice A is correct. The trait displays complete penetrance, as all individuals in the ancient population who have inherited the genotype display some degree of resistance to hypobaric hypoxia (choices C and D are incorrect). The trait also displays broad expressivity, as there is a wide variance in the resistance to hypobaric hypoxia that exists (choice A is correct).
-----
Part 7: Standalone questions and answers
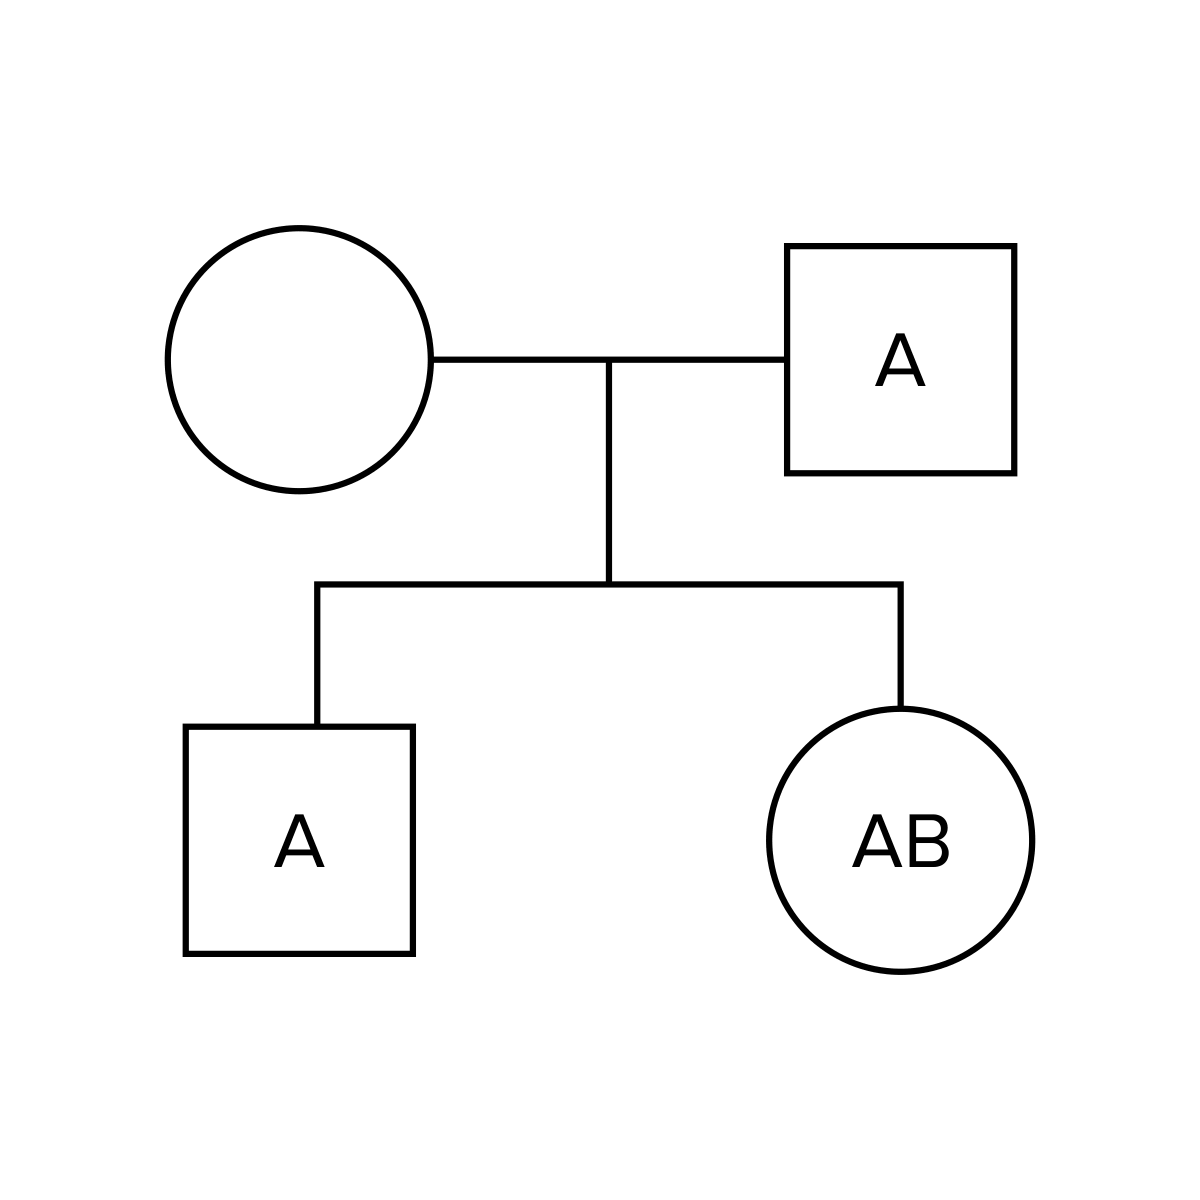
Question 1: The following pedigree shows the blood types of two children and their father under the AB system. What is one possible maternal genotype?
A) ii or IAi
B) IAi or IAIA
C) IBIB or IAIB
D) IBi or IAIB
Question 2: In the pedigree shown below, individuals affected with an inherited disorder are shaded in black.
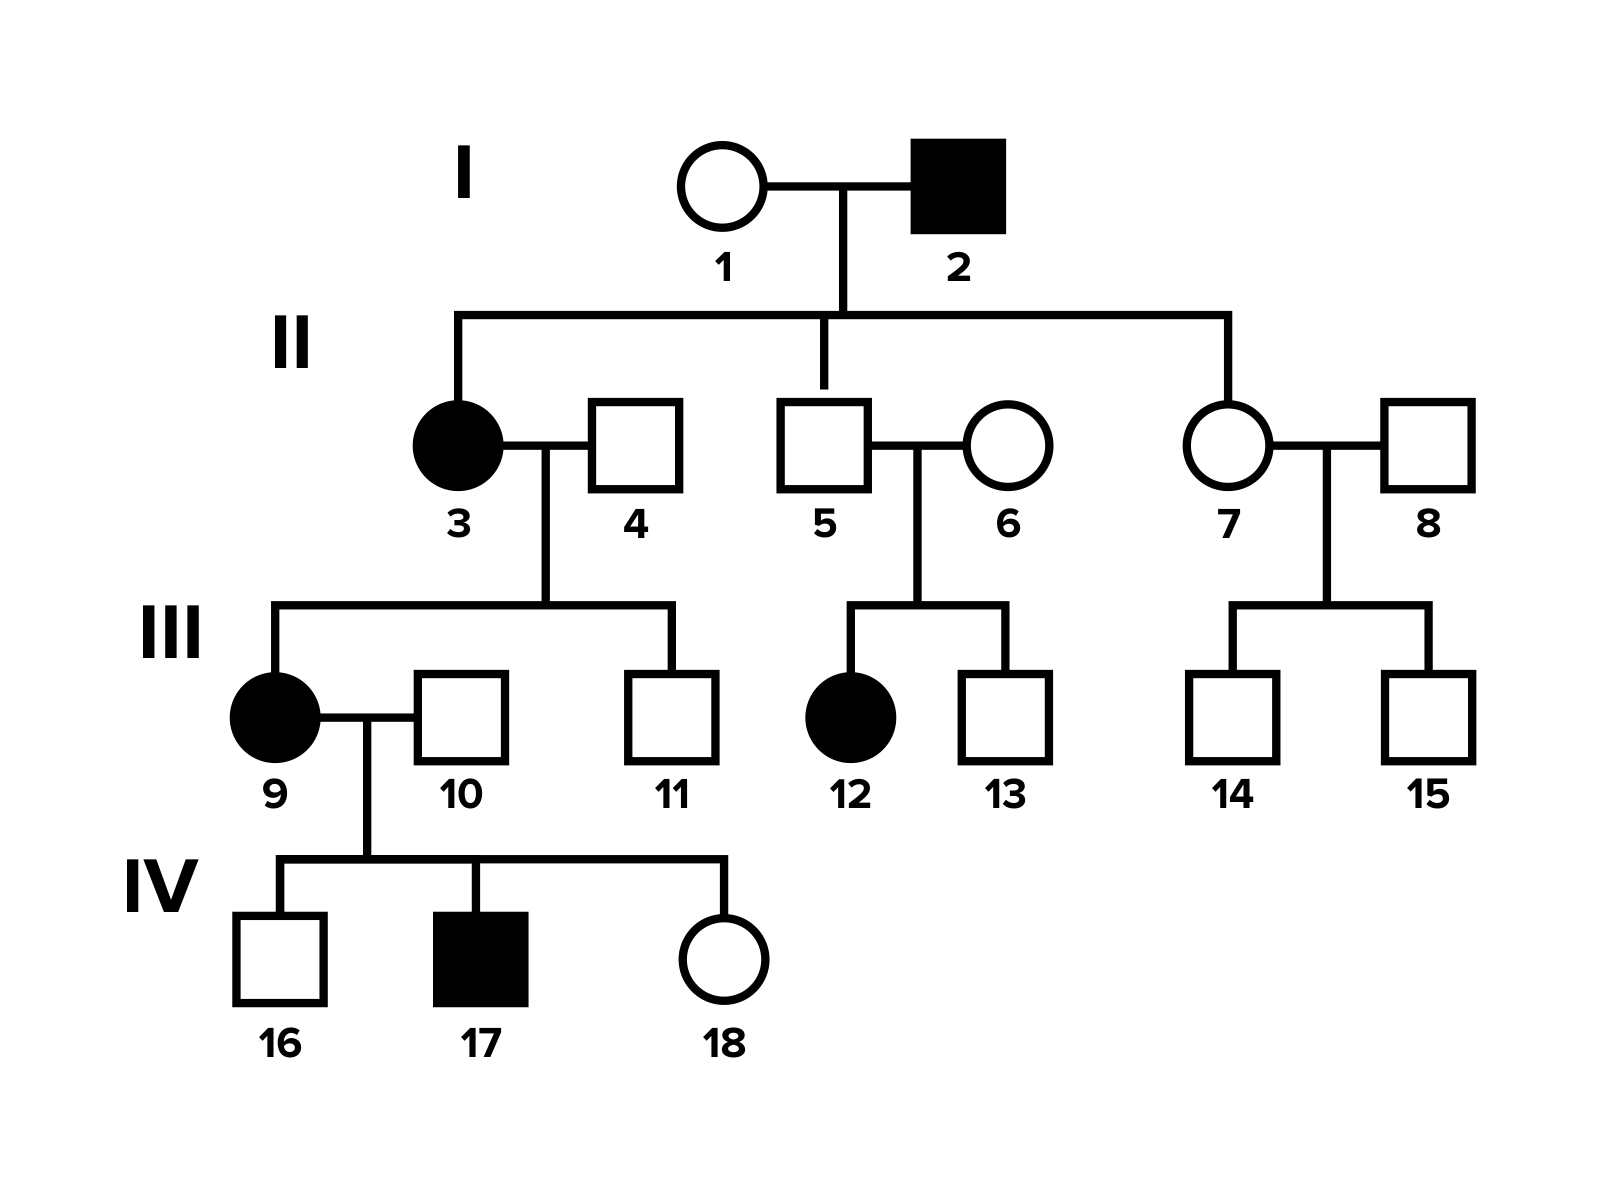
What is the most likely mode of inheritance of the mutation?
A) Autosomal dominant
B) Y-linked dominant
C) X-linked recessive
D) Autosomal recessive
Question 3: In fruit flies, the autosomal vestigial gene has a dominant V allele that produces long wings and a recessive v allele that produces vestigial wings. The autosomal striped gene has a dominant S allele that produces striped bodies and a recessive s allele that produces smooth bodies. A heterozygous female fly with long wings and striped body mates with a homozygous male fly with long wings and smooth body. What is the expected genotypic ratio in the offspring?
A) 9 VVSS : 3 VvSS : 3 VVSs : 1 vvss
B) 1 VVSs : 1 VVss : 1 VvSs : 1 Vvss
C) 1 VVSs : 2 VVss : 1 Vvss
D) 9 VVSs : 3 VVSs : 4 VvSs
Question 4: A population of birds lives on an isolated island. Which of the following events are least likely to disrupt the equilibrium of their gene pool?
A) Relatives from the mainland arrive via a passing boat and mate with the island birds.
B) Male birds with orange plumes on their head are more successful in their mating rituals than birds with yellow plumes.
C) Hunters arrive and spot the birds with orange plumes most easily.
D) The birds never nest on the tree they were hatched in.
Question 5: The frequencies of genotypes at an autosomal locus are as follows:
| Genotype | MM | MN | NN |
| Number of individuals | 10 | 20 | 20 |
What is the predicted genotype frequency of the MN genotype in the next generation, assuming random mating occurs and no genotype is selected for or against?
A) 0.24
B) 0.25
C) 0.48
D) 0.50
Answer key for standalone questions
- Answer choice D is correct. In pedigrees, male individuals are represented by squares and female individuals are represented by circles. Given that IA and IB alleles are codominant, the daughter’s blood group was AB, and the father’s blood group was A, this indicates that the mother must have had at least an IB allele (choices A, B, and E are incorrect). The son’s blood type was A, which is possible through either an IAi or IAIA phenotype. Thus, at least one of the maternal alleles must be IA or i (choice C is incorrect.)
- Answer choice D is correct. The condition is able to skip generations (such as in the case of individual 12), indicating that the mode of inheritance is recessive (choices A and B are incorrect). The condition is not passed from the affected female 9 to her son 16, which indicates that the condition is not X-linked. Otherwise, all of individual 9’s male offspring would be affected (choice C is incorrect).
- Answer choice B is correct. The parental genotypes here are VvSs (female) and VVss (male). The female can generate VS, Vs, vS, and vs gametes with equal frequency, while the male can only produce Vs gametes. The following Punnett square for a dihybrid cross can be drawn:
♂\♀ VS Vs vS vs Vs VVSs VVss VvSs Vvss Vs VVSs VVss VvSs Vvss Vs VVSs VVss VvSs Vvss Vs VVSs VVss VvSs Vvss
The offspring are thus expected to share a 1:1:1:1 ratio of VVSs, VVss, VvSs, and Vvss genotypes. (Note that this implies that 100% of the offspring will have long wings, while 50% of the offspring will have striped bodies and 50% of the offspring will have smooth bodies.) - Answer choice D is correct. To achieve Hardy-Weinberg equilibrium, five conditions must be met: random mating individuals, no selection, large population, no gene flow, and no mutation. Immigration of individuals disrupts gene flow (choice A is incorrect). Sexual selection mate selection prevents random mating (choice B is incorrect). Discriminative hunting presents a selective force (choice C is incorrect), while the nesting preferences of the birds do not necessarily prevent the mixing of the population (choice D is correct).
- Answer choice C is correct. The total population of individuals is 50, and these are diploids, so 100 copies of the gene locus exist in total. Of these, the frequency of M alleles is (10x2) + 20 = 40, so the allelic frequency of the M allele is 40/100 = 0.4. Using the formula p + q = 1, the allelic frequency of the N allele is 0.6. Since the Hardy-Weinberg conditions are met, we can use the formula p2 + pq + q2 = 1 to determine that the genotype frequency for MN must be equal to 2pq = 2 x 0.4 x 0.6 = 0.48.
Not ready to commit to your MCAT prep at this time?
Enter your name and email for a free MCAT question delivered straight to your inbox daily.